The buzz on neonicotinoids

Picture1
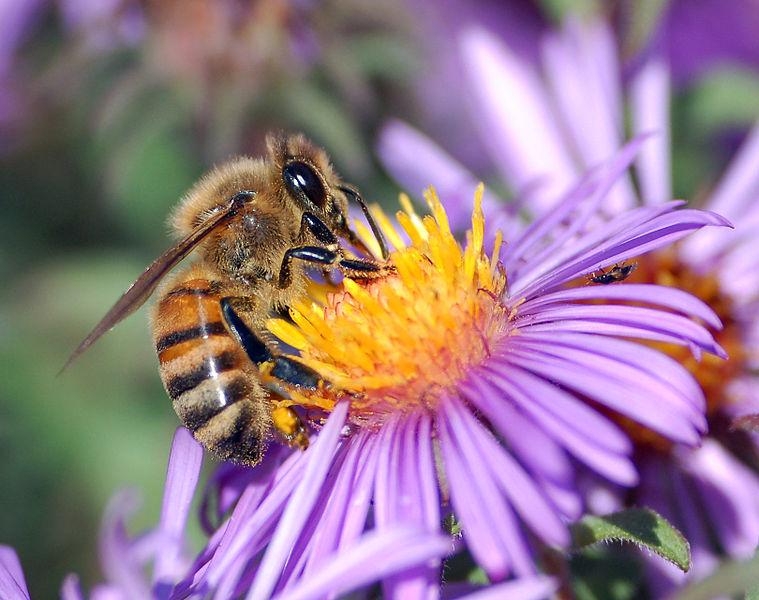
On the 31st January, stimulated by a European Food Safety Authority report, the EU proposed banning three neonicotinoid insecticides which have been implicated in causing honeybee decline. These insecticides are widely-used, systemic (i.e. soluble enough in water to move around the plant’s vascular system to nearly all plant tissues), and, like nicotine, affect the insects’ central nervous system. They are highly effective at reducing insect pests that feed on crops and reduce yields and value, and many farmers are concerned about the effect the proposed ban will have on crop production. But these insecticides can also end up in the nectar and pollen of crops (as well as in the soil and in non-crop plants), and thus can have unintended side-effects on beneficial, nectar-feeding insects, who act as pollinators. Especially bees.

Bee decline has become a hot topic with scientists, the media, the public and even some politicians, but until recently the threat of neonicotinoids to bees has not been seriously implicated in their decline. Concern about pollinator decline is a result of the important role that pollinators play in food production: 75% of crop species depend on animal pollinators, which translates into 35% of global production; and the total annual economic value of pollination has been estimated at €153 billion globally. In addition, pollinators are fundamental to most terrestrial ecosystems, and indirectly affect the availability of food for other organisms (e.g. fruits and berries for frugivorous birds), as well as the structure and functioning of ecosystems.

So here’s the paradox: flower-visiting insects including bees are really important for agricultural production. But so is the use of neonicotinoid pesticides. Which is more important and is the ban justified on scientific grounds?

In the last year, the evidence that neonicotinoids have negative impacts on bees has been mounting. Bees and other flower-visiting insects are exposed to neonicotinoid pesticides in multiple ways: during planting of seeds which have been coated with pesticides as a pre-planting treatment, by collecting pollen and nectar from the crop, and by foraging on non-crop plants which take the pesticide up through the soil. Traditionally, toxicological tests of agrochemicals are carried out on the managed honeybee Apis mellifera, and pesticides are rated according to their lethal effects (by calculating the LD50 – the dose required to kill half the organisms tested after a specified duration). But the biology of Apis and all the other bee species (20,000 of them worldwide) is different. Can we generalise about effects on Apis, to effects on other bee species, and other pollinating insects including hoverflies and butterflies? And what about sub-lethal effects, i.e. those that don’t kill the insects, but affect their physiolology, behaviour and fitness?

Neonicotinoids are highly toxic to insects – that’s the whole point of them. Bees are insects. So it shouldn’t be too much of a shock that they kill bees. Last year it was shown that neonicotinoids can also have sub-lethal effects in honeybees, by decreasing foraging success and navigation by individuals back to the hive. At the same time, the neonicotinoid pesticide, imidacloprid, can reduce bumblebee colony growth and fitness by affecting their feeding behaviour. Some dissenters have cast doubt on the field-relevance of laboratory tests, claiming that field-realistic dosages have not been used, but this is not the case – the concentration of imidacloprid in oilseed rape flowers for example has been found to be 4.4-7.6 mg/kg in pollen and 0.6-0.8 mg/kg in nectar, which was within the range tested on bumblebees. This is pretty convincing evidence that neonicotinoids can cause very adverse effects on populations of these social bees.

Although neonicotinoids are not the only cause of widespread bee decline, they are more than likely contributing to it. Some of the agrochemical companies are claiming that bee decline has nothing to do with their chemicals and instead blame decline on Varroa destructor, the parasitic mite which infects honeybee colonies. Whilst Varroa probably plays its part in honeybee decline, the most probable cause of decline in other bee species is multiple pressures, including habitat loss and loss of forage plants, AND the use of neonicotinoid pesticides.

So should these insecticides be banned? YES, if we want to address pollinator decline. They should not be used for insect-pollinated crops, and wind-pollinated crops that insects forage on (including maize). But what’s the alternative for the farmer? How can crop production be maintained in the absence of these chemicals? Use something worse? If we’ve learned anything since Rachel Carson’s “Silent Spring” published 50 years ago last year, it’s that an alternative will be found, and we can’t be sure that this won’t be worse for the bees and other pollinating insects.

Author

Jane Stout: stoutj@tcd.ie

Photo credit

wikimedia commons
Sampling gaps in our understanding of primate parasites

Jigokudani_hotspring_in_Nagano_Japan_001

*by parasites here I am referring to all kinds of infectious disease causing agents including bacteria, viruses, fungi, protozoa, helminths and arthropods.

Why do we care about primate parasites?

Many of the most devastating infectious diseases in humans have origins in wildlife. For example, the global AIDS pandemic originated through human contact with wild African primates and influenza viruses circulate among wild bird populations. These are not only historical occurrences. Recently, for example, rodents were identified as the source of a Hantavirus outbreak in Yosemite National Park, USA . As human populations continue to expand into new areas and global changes in temperature and habitat alter the distributions of wild animals, humans around the world will have greater contact with wildlife. Thus, understanding which infectious agents have the potential to spread from animals to humans is crucial for preventing future human disease outbreaks.

Many efforts are being made to collate information on wildlife and human diseases. Much of my research (which I will blog about when I get chance!) uses an amazing database known as the Global Mammal Parasite Database or GMPD for short. Every time a paper is published which contains details of parasites found in either primates, carnivores or ungulates, the information is added to the database. As much data as possible is recorded, including the species infected, the type of parasite, the prevalence of the parasite, and the geographic location of the study. Prof. Charles Nunn and his colleagues have been collecting data for the GMPD since around 2005 and it currently contains around 6000 records for primates alone. This definitely makes it the most comprehensive dataset of primate parasites in existence.

The GMPD sounds amazing…so what’s the problem?

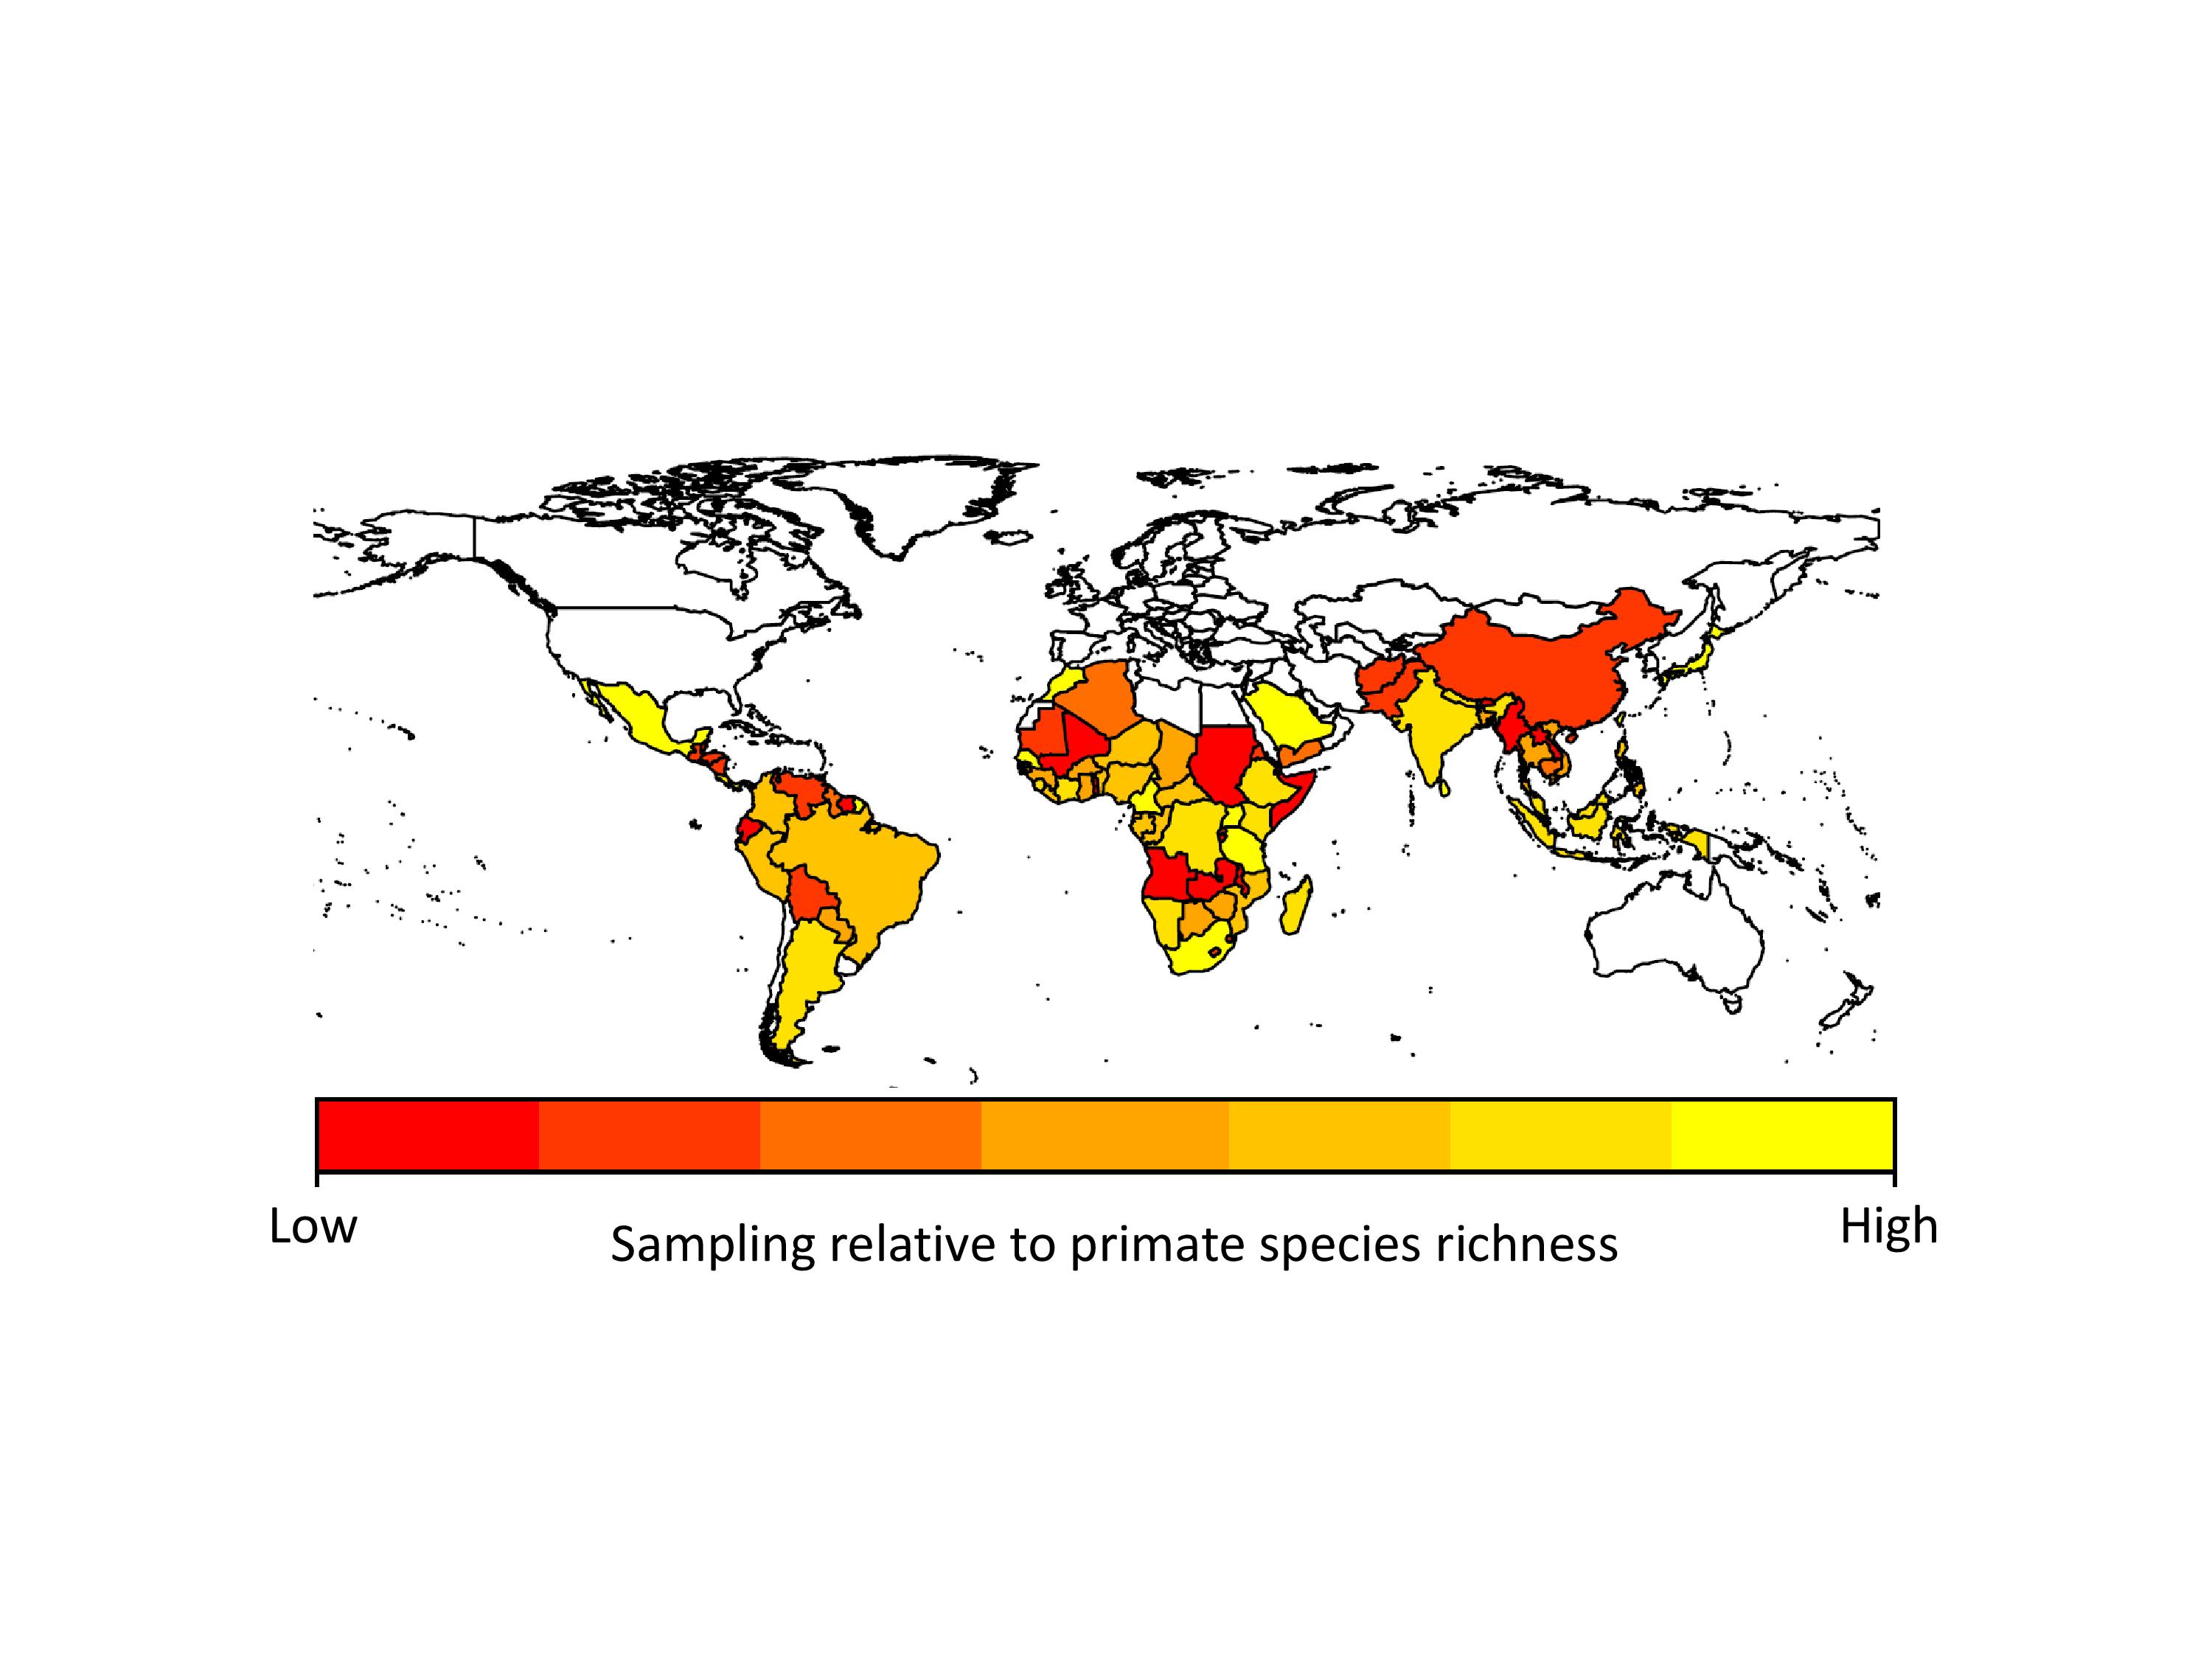
The problem with the GMPD (and this is a feature of virtually all datasets) is that there is sampling bias. Certain primates are sampled for parasites much more frequently than others. Chimpanzees, for example, are sampled for parasites all the time, whereas species such as tarsiers are sampled much less often. This has the effect of making it look like chimpanzees have far more parasites than tarsiers, simply because they have been sampled more often. In analyses using the database we usually deal with this problem by adding sampling effort into our models, so we give less emphasis to high numbers of parasites in primates we have lots of samples for. Unfortunately this problem is also evident when we look at parasites (things like malarial parasites are often sampled because of their importance to human health) and geographic regions (areas with primate research stations are sampled far more regularly than more remote regions). If we hope to use the GMPD data to make reliable predictions about future risks to humans, we need to identify gaps in our knowledge of primate parasites.

So what did you do?

Without going into the technical details, we looked across the primate phylogeny and primate geographic ranges to identify gaps in our knowledge, and used statistical models to investigate what factors led to primates and geographic areas being relatively well- or relatively poorly-sampled. We also used species accumulation curves to extrapolate parasite species richness for primates.

Where are the gaps in our knowledge?

We found that apes (chimpanzees, gorillas and orangutans) were generally better-sampled than other primates, but there was incredible variation in sampling among all other major primate groups. Apart from apes, the primates that researchers appear to sample most are the species they encounter most often, i.e., widespread, terrestrial, diurnal species. However, some primates were sampled more often because they are already intensively studied for other research, because they live in frequently visited field sites, or because of their importance in medical research. Across countries, we found that in general, parasite sampling is highest in countries with more primates to sample. We expected that the GDP of the countries would also affect sampling effort, with wealthier countries having more money for disease monitoring. However, we found no evidence for this in our analyses, probably because most research on primate diseases is not funded by the country in which the research takes place.

Sampling effort for primate parasites across the world. Poorly-sampled countries are in red, and better sampled countries are in yellow.

When we extrapolated parasite species richness values we found that even within our best-sampled primates and countries, we are missing a lot of parasites. On average we predicted that 38-79% more parasite species than currently reported in the GMPD should be found in our best sampled primate species, and 29-40% more parasite species than currently reported in the GMPD should be found in our best sampled countries. This emphasizes exactly how poor our sampling is across all primates and countries. Another concern is that although viruses make up only 12% of the parasites in our dataset, viruses arguably present the greatest zoonotic disease threat to humans because their fast rates of evolution should allow them to easily adapt to new hosts.

What next?

Identifying parasite sampling gaps across primate species and geographic regions is only the first step; we need to find strategies to minimize these sampling gaps if we are to predict which primate diseases may emerge in humans. One solution is to set research priorities based on the sampling gaps, for example, by focusing effort and funding on relatively poorly-sampled primate species, arboreal primates, those with small geographic ranges, or those found in relatively poorly-sampled regions of South East Asia, Central and Western Africa, and South America.

Focusing on relatively poorly-sampled primate species and areas may improve our general understanding of primate parasites, but it is only one factor in predicting risk to humans. For example, hosts are more likely to share parasites with their close relatives than with more distant relatives. Thus, continuing to focus our sampling efforts on parasites of our closest relatives (chimpanzees, gorillas and orangutans) may provide the greatest return in the case of risks to humans. This is particularly important because we found that chimpanzees are expected to have 33-50% more parasites than currently found in the GMPD. In addition, ecological similarities also influence parasite sharing among primates, and humans share more parasites with terrestrial than arboreal primate species. As with sampling effort, this probably reflects higher contact rates among humans and terrestrial primates compared to arboreal primates. As a related issue, a host living at higher density is expected to have higher prevalence of parasites and may have more contact with human populations or our domesticated animals, thus increasing opportunities for host shifts to humans. The large numbers of zoonotic emerging infectious diseases with rodent or domesticated animal sources also highlight the importance of rates of contact and host density for disease emergence in humans.

In conclusion Sampling effort for primate parasites is uneven and low. The sobering message is that we know little about even the best studied primates, and even less regarding the spatial and temporal distribution of parasitism within species. Much more sampling is needed if we hope to predict or prevent future emerging infectious diseases outbreaks.

Author

Natalie Cooper

nhcooper123

ncooper[at]tcd.ie

Photo credit

Natalie Cooper, wikimedia commons

Coursing conundrum

Female_Irish_mountain_hare

At first glance, many scientific ideas can appear counterintuitive. A press release from a leading Irish wildlife charity in support of the proposed coursing ban prompted me to attempt to balance the discussion of coursing impacts on the Irish hare population. The bill to ban coursing is due to come before the Dáil in the coming months. However, the above press release immediately struck me as biased, and so I felt a discussion of coursing impacts was required before the public were asked to sign any petitions in support of this ban. For those unsure of just what coursing is, it is a popular field sport which consists of a hare being chased by a pair of greyhounds over a short distance. Unlike fox and deer hunting, the aim of coursing is not to kill the hare. It is instead a speed and agility competition between two dogs, where each is awarded points depending on its ability to “turn” the hare from a direct route along the field. Irish hares (Lepus timidus hibernicus Bell 1837) are caught and held in captivity prior to an event during which the hare is coursed within an enclosed park. A running hare is given a 75m head start before the release of two dogs, whose performance is assessed by a judge, and surviving hares escape into an area from which the dogs are excluded. The duration of the pursuit is relatively brief, usually lasting less than a minute, and surviving hares are returned to the wild after the event.

The IWT states something which a few of us may agree with; that Ireland is lagging behind in terms of its attitude to welfare and conservation of native wildlife. However, the idea that a coursing ban would in some way improve this status is highly questionable. Welfare issues need to be taken into account, but these considerations must be viewed in parallel with the beneficial aspects of coursing, such as habitat conservation and the associated protection of both target and non-target species, before any final judgements regarding coursing acceptability can be made. It is perhaps unintuitive, but evidence indicates that coursing has an extremely large positive impact on hare numbers. Mortality of coursed hares stands at just 4.1% since the implementation of dog muzzling in 1993, and research has found coursing to have negligible impacts on hare populations due their large intrinsic rates of increase. People who participate in coursing maximise hare populations in coursing preserves through predator control and set aside to conserve habitat suited to the Irish hare. In fact, it is agricultural intensification (an issue completely ignored in the IWT article) which is more likely to blame for population declines. Habitat management to encourage target species for hunting can protect against the detrimental effects of modern agricultural policy on biodiversity. Irish Coursing Club preserves host a hare density 3 times greater than that supported by the wider countryside. What is more probable is that coursing is actually stemming the tide of anthropogenic destruction of many species our native wildlife (including corncrakes and many other farmland bird species) through habitat conservation aimed at artificially increasing hare populations for coursing. If coursing were to be banned in this country, this practice would be completely abandoned due to waning interest in encouraging hare numbers, and could potentially have serious ramifications for other wildlife which benefit from associated habitat management and predator control. Incentives to promote hare conservation would be required, but it’s questionable whether these would produce the same results as coursing-associated management due to a lack of personal interest for farmers and other landowners who practice coursing. Hare conservation in the absence of coursing, similar to that of other species benefiting from game management, would be a costly endeavour and would be unlikely to be awarded the necessary funding in the Republic of Ireland with the current economic climate.

We have the opportunity to be forward-thinking, innovative and inclusive in the way in which we achieve sustainable conservation of our native wildlife, something which appears all the more important in light of the EU agricultural policy reforms which were leaked in recent days. We can only hope that a review of the research will stop the Dáil bowing to ill-informed political pressure and perhaps, the future of farmland birds and our only endemic mammal, the Irish hare, will be ensured.

Author

Emma Murphy: butlere1[at]tcd.ie

Photo credit

wikimedia commons
The Flora of the Future

Flora of  the future

It’s the year 2050. Several billion more humans occupy the world, and species translocations are by now the norm to mitigate against increased urban sprawl, climatic instability and a sea level now a third of a metre higher. In spite of unprecedented demands on the natural environment, governments have slowly developed capacity for conservation of wilderness and semi-natural habitat. Beyond this even, with the vast majority of the human race by now living in cities and the continued trend of rural land abandonment; restoration ecology has come to the fore at entire landscape and regional scales. The concept of ‘rewilding’ is debated openly amongst politicians and the public – no longer the mere theoretical exercise of academics. The monetary value of ecosystem services is also by now a very real and tangible concept within economic circles, embedded within highly developed metrics such as green-GDP.  Despite such positive developments, however, problematic legacies of the past remain. Intensification of agriculture has been unrelenting globally, notwithstanding inroads into adoption of agroecosystem approaches. A transition to truly renewable energy sources is still incomplete and of utmost urgency. One of the most critical questions of all most likely still looms – have we yet done enough to put a cap in the peak of this, the sixth great mass-extinction of life on the planet?

And so, it is within this future and none-the-less challenging world we find the modern ecologist and biodiversity practitioner at work.

What kind of new and useful technologies may exist to help tackle such problems and challenges of the not so distant future? It is interesting to deliberate on one low-tech tool in particular (the so-called bread and butter of biodiversity), which has been with us already for centuries – and that is the humble species checklist. Specifically we take a look at the Flora – and although coverage here is rather phyto-centric, it should be easy to draw equivalents to all forms of taxa, without (too) much stretch of the imagination.

So what is a Flora in the traditional sense, why is this changing, and how will the Flora of the Future look and function? To briefly tackle these first two questions, a Flora is primarily a list of plant biodiversity (either with or without diagnostic characters and keys) within a specified geographic range, be it local, national or at larger scales. Outside of this basic function there are the ‘added-extras’, which may include notes on distribution, ecology, synonymy, conservation status and even ethnobotanical use. Often the assemblage of national-level Floras has proven quite a mammoth task; logistically challenging, fraught with funding difficulties, and above all time-consuming – with efforts spanning over several decades for particularly biodiverse countries. This is all very well, and such traditional Floras have and will continue to serve as invaluable tools. In this modern age, however, change is called for to tackle some common short-comings of the Flora.  A considerable amount of valuable information collected by taxonomists and other experts in the production process is typically lost, never making its way into the public realm – and when such publications can easily run to over 20 volumes, it is clear to see the major constraints involved. Another key drawback is the sheer speed at which redundancy can occur. Even before the final volume of a Flora is published, taxa (species/genera/families) covered within the first volumes may have long been ripe for new taxonomic treatment.

The revolution in how biological information is collected, stored and disseminated is already greatly influencing the Flora. One of the most recently initiated national-level projects is the Flora of Nepal project, for which advances in biodiversity informatics have permeated the entire process from preparation to publication. Although the Flora of Nepal will still be published in printed format, a (if not the) main focus will be an E-Flora freely accessible online, which will also greatly expand the availability of information assembled by experts. A simple yet very significant feature will be the ease of portability of numerous volumes to the field in digital format.  Though perhaps most critically, the Flora of Nepal will be maintained and updated to reflect new findings – creating for the first time, in essence, an evolving Flora.

Before we really begin to speculate on the form and function of our Flora of the Future, we must first take a look to the current cutting edge of biodiversity informatics. In what must be one of the most significant advances in decades, the cooperative development of the Global Biodiversity Information Facility (GBIF) by many governments and organisations has promoted and facilitated the “mobilization, access, discovery and use of information about the occurrence of organisms”. This centralized repository of earth’s biodiversity is fast set to reach one billion indexed records within a few years from now, fed from diverse sources ranging from individuals to national biodiversity data centres. It is difficult to envisage how the Flora of the Future could in any plausible way side-step such a global network. Whereas floras have traditionally featured a top-down, expert driven synthesis – the Flora of the Future will also no doubt integrate the emergent trend of bottom-up assembly of knowledge – a good example of which is currently purveyed by the Encyclopaedia of Life.

Let’s get back now to our future ecologists and biodiversity practitioners, and take a little look in as they go about conducting their fieldwork. No matter what habitat or location they study in worldwide, they will each possess a small handheld device connected to the Flora of the Future. Automation of species identification by means of this device will have removed a large bottleneck in their work – leaving ecologists to focus on actual ecology. No longer will they be bound to a particular geographic territory due to limited floristic familiarity –  we will witness a complete opening of boundaries, and greater migration of ‘western’ ecologists to the frontline of areas of global biodiversity importance.

But just how exactly could such a device work? A potential basis could feature a combination of machine-learning morphometrics and DNA barcoding  – two presently very promising tools. For the former, development of algorithms for auto-identification of plant species is already well underway (see for example the Leafsnap mobile app). These function much like facial recognition technology, and through input of a digital scan/photo can pinpoint unique morphological characteristics required for successful classification. A key aspect of machine learning is removal of subjectivity by conversion of shapes into numerical descriptions – no need for argument any longer on just how ‘subglobose’ a feature is; the ball is already in motion towards a predictive and integrative taxonomy. Upon scanning a specimen in the field, an image will be broken down into key morphometric characteristics, and referenced against a large central database within the Flora of the Future. The Flora will prioritize this procedure by first referencing against species known to occur within a certain radius from where the user currently stands (a useful feature in itself!). The ecologist, on the spot, may learn that the specimen has a confirmed match, and proceed to download key local statistics of importance. On the other hand, this specimen may in fact represent an extension of the species known distributional range. The finding, however, of no known match in the database could spell discovery of a new species, whereas a positive match with notably low morphometric agreement may indicate new subspecific taxa or otherwise interesting findings (for which DNA barcoding could be employed for further verification in both cases).

Regardless of outcome, the above three scenarios will have allowed for a real-time and in situ solution to identification of species. The exact significance of this process will not only lie in the freeing up of both ecologists’ and taxonomists’ resources, but in the real-time flagging of new discoveries. As it stands, it is expected that discovery of remaining undescribed plant species will be an incredibly inefficient process (given that 50% of the world’s plant species have been discovered by only 2% of plant collectors), despite the vast number of these thought to exist. A recent study examining the exact inefficiency of the production chain from collection to publication uncovered that “on average, more than two decades pass between the first collection of samples of a new species and the publication of the species’ description in scientific literature”. In other words, a specimen of a new species has physically passed through the hands of many people before the simple ‘discovery’ (perhaps after many, many years in a herbarium) that it is something new to science. In this sense, an important function of the Flora of the Future will be instant recognition (perhaps even while standing in the field!) of a new discovery as just that – which can drastically reduce this presently overblown timeframe and waste of resources.

Getting back to the future for now, we see our biodiversity practitioners and ecologists as key players in the advancement of ecological as well as taxonomic discovery, with a highly efficient yet passive ability for discovery embedded within the commonplace tools they use, as they go about their work.  With an entirely streamlined approach to field research, and identification no longer a daunting prospect in the study and documentation of biodiversity, we will eventually see the peak of mass extinction pass, looking back behind us. The challenges of tomorrow are no doubt great, and a renewed vigour for the taxonomic process will be critical for progress on these fronts. The Flora of the Future will for the first time sew a seamless line between ecologists and taxonomy; the essential currency of biodiversity.

Author

Paul Egan: eganp5[at]tcd.ie

Photo Credit

Paul Egan

Another piece in the trophic puzzle

Meles.meles

The food chain is a concept that many non-biologists are familiar with. Ecologically-speaking, this should be referred to as a food web, because there is rarely one prey species for a given predator or one predator of any given species.

The biochemistry of metabolism and digestion means we can reconstruct the diet of a member of a given food web with some basic information about the stable isotopes in its tissues and the stable isotope values of the available prey. Simply put, “you are what you eat”. Carbon isotopes generally reflect the “where” of the diet and nitrogen isotopes generally indicate the “what”.

This overview omits several complications. Firstly, the calculation of diet requires a “conversion factor” (trophic enrichment factor or TEF) for any given tissue of an animal. Animal metabolisms tend to retain 15N, so consumers have greater 15N:14N ratios than their prey. Secondly, each tissue is likely to have a different TEF, as it is made to perform a different job in the animal. Thirdly, TEFs can only be derived by feeding animals highly controlled diets, ideally a single food for the length of time it takes for the study tissue to be fully replaced. In the case of teeth and bone, this can be months or even years.

As there are relatively few TEFs available for animal species, many ecologists “borrow” TEFs from other species for their calculations. Having derived TEFs for carbon and nitrogen in badger blood serum, a tissue that is completely replaced several times a month, we demonstrated that badger TEFs differ from fox TEFs. This is important, as foxes are similar in size to badgers and have a similar feeding ecology, and ecologists might be tempted to “borrow” fox TEFs to use in badger studies.

So knowing more about the biochemistry of badgers (in the form of TEFs) will allow us to learn more about their diets. This may be of importance to farmers planning biosecurity measures for their farms, as they will be able to learn if badgers are raiding their crops (in the field or in the barn). It will also help identify when badgers are specialising on different foods and potentially allow farmers to minimise contact between badgers and livestock.

Authors

David Kelly: djkelly[at]tcd.ie

Nicola Marples

Photo credit

wikimedia commons

City slickers

Urban_wildlife_-_squirrel

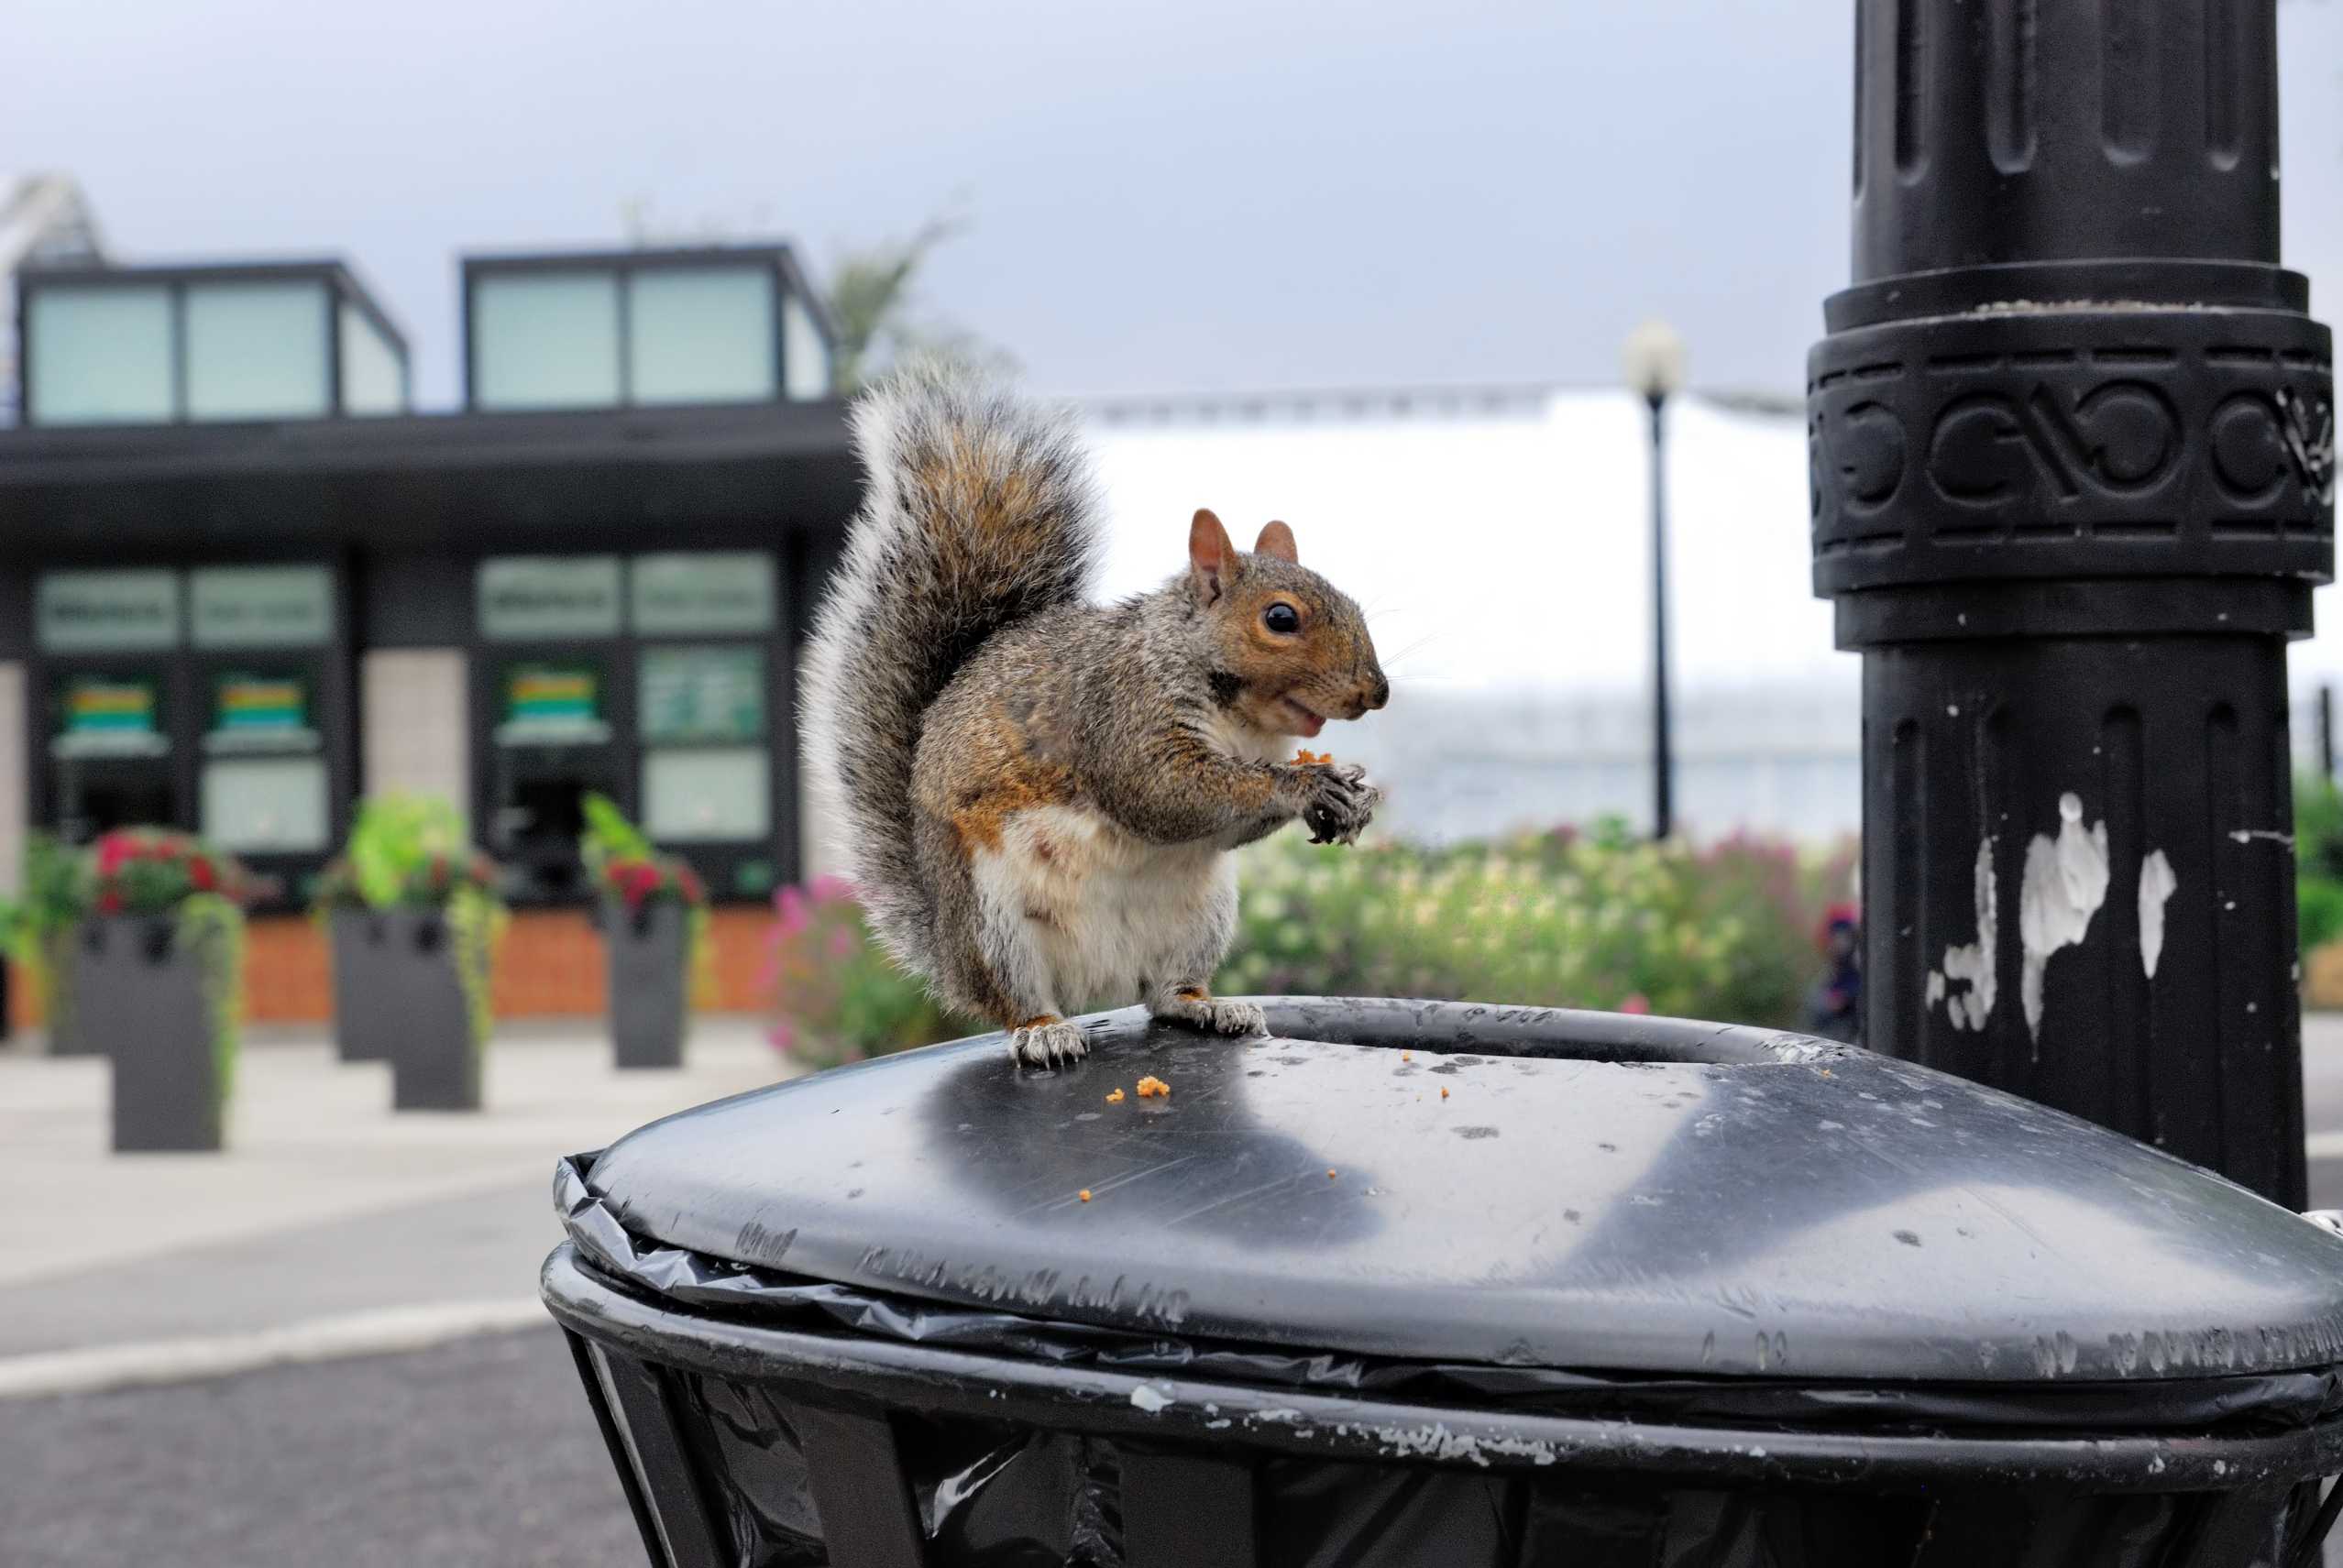
Typically, when humans and wildlife meet it’s curtains for the latter. Think of all the megafaunal extinctions in the past and the mounting evidence that we’re responsible for an ongoing sixth mass extinction event. Aside from directed extermination we can change the environment over a very short time-scale to suit our needs and other lifeforms are often left playing catchup. This is especially true for plants and animals (microorganisms have such short turnovers that we don’t really impact them in this way); the plight of the blue swallow isn’t top of an industrialist’s list of priorities.

Despite these radical changes, some species have adapted to living in our towns and cities. This has piqued the interest of scientists and we’re now seeing the burgeoning field of urban ecology populated by urban ecologists. The amount of urban biodiversity is quite surprising and the adaptations of the flora and fauna comprising it equally so. Look at the previous post talking about birds lining their nests with material from discarded cigarette butts.

As civilization has developed we’ve become more aware of the value of nature, be it an intrinsic worth or a more practical value. So we can actively change our urban centres to accommodate more species if and when we choose. Sushinsky and colleagues asked how we should grow our cities in order to minimise their biodiversity impacts. Their conclusion was a more concentrated city plan would be better suited to avian diversity than a sprawling one. Certainly, it seems better for our cities to grow vertically rather than horizontally if we are to minimise humanity’s footprint. So, more New Yorks and fewer Los Angeles.

We can even provide supplementary food to animals. Fuller et al. showed that bird feeders can increase the abundance of birds and pointed out that up to a third of households in Australia, Europe and North America supply food for birds.

Then there are species that can prosper on our discards when it hasn’t been our intention to feed them in the first place. Badgers, foxes, raccoons, bears, the list goes on. All of them can make a living in an urban setting.

With more and more of us cramming ourselves into cities we should be aware that there are real benefits to interacting with nature. We feel psychologically better when there is more of the natural world around us.

To butcher Gordon Gecko, green is good.

Author

Adam Kane: kanead[at]tcd.ie

Photo credit

wikimedia commons
No animal is an island

800px-Impala_mutualim_with_birds_wide

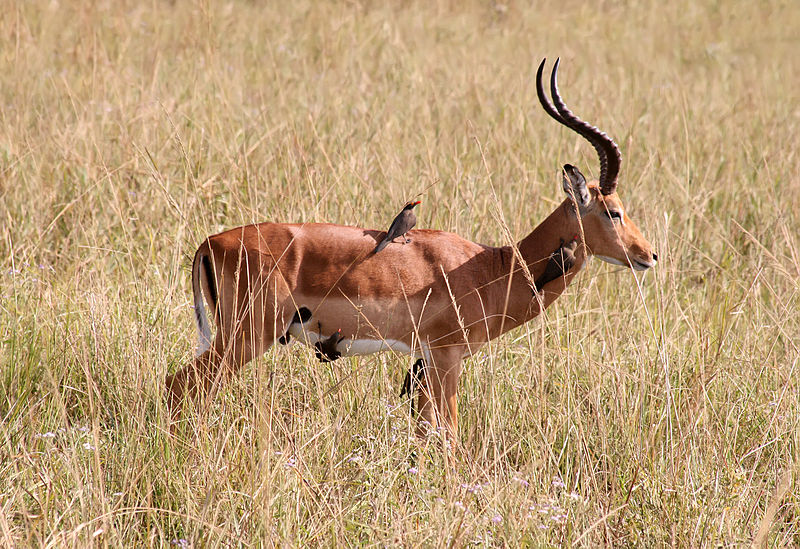
No man is an island; the same could be said for the millions of life forms that populate our planet. Think of all the ways in which organisms interact with each other through predation, parasitism and the countless symbioses. Sometimes a pair of interacting partners can become inextricably linked such is their mutual dependence. Each one may provide the other with a resource it’s unable to obtain on its own.

A recent collaboration explored instances when these interactions lead to the loss of a trait and showed the fragility of this situation. One of the examples the authors use is an ant species that farms fungus. The fungus provides the ants with all the arginine (an amino acid) they need so they have lost the ability to synthesise it themselves. Thus anytime an ecological interaction involves some provision of a resource by one partner to another the evolutionary pressure is removed and the trait can be lost in the species receiving the goods.  In other words we end up getting ‘compensated trait loss’ due to the ecological interaction. This can tighten a symbiosis from a facultative to an obligatory one.

But the fragility of compensated trait loss should be obvious now. In the ant example, were the fungus to go extinct the ant would disappear along with it. It’s like the ecological interaction is undermining all the good work done by natural selection in providing the ancestral ants with all the traits they need. The authors reckon that trait loss is “grossly underestimated” which puts many species in a precarious position in this age of mass extinction. Although there have been some instances where the trait was recovered, in flagrant disregard for Dollo’s law. Some of these law breakers include parasitic insects who regained their ability to synthesise lipids once the provision was lost.

A difficulty in studying these systems is how to detect when trait loss is taking place. A decreased expression of some gene in some members of a population would probably be reported as natural variation. But with ever improving molecular techniques we will be able to get a better estimate of the number of compensated trait loss interactions.

Author

Adam Kane: kanead[at]tcd.ie

Photo credit

wikimedia commons
Smoking nests

769px-Filthy_Habit_by_SillyPuttyEnemies

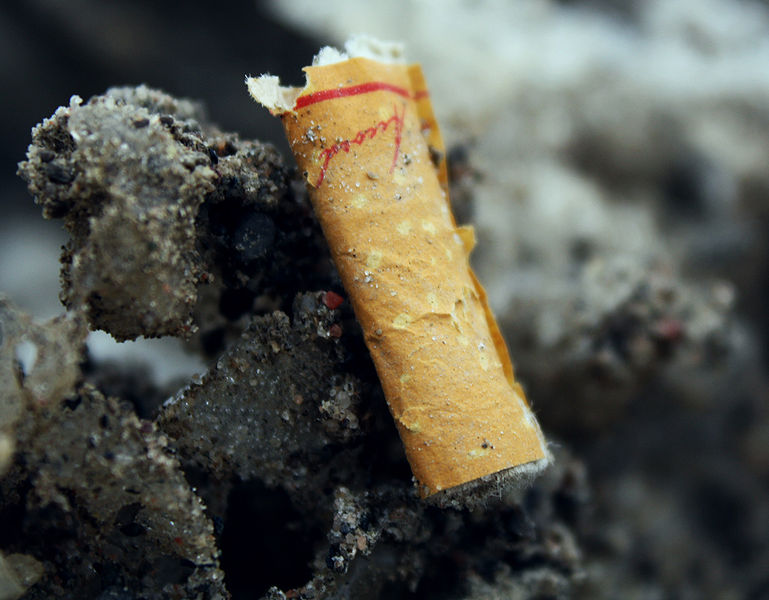
We all know that cigarettes and smoking are bad for you. However, a recent Biology Letters paper which was featured on BBC Nature suggests that the discarded remains of cigarette butts may help to maintain the health of some urban birds.

Researchers from the National Autonomous University of Mexico found that smoked cigarette butts incorporated into house sparrow and house finch nests may act as parasite repellents. Nests which included high numbers of cigarette butts had fewer parasites. A further experiment involving heat traps to attract parasites indicated that the anti-parasitic properties of the cigarettes seemed to be related to their nicotine content which is only released after the cigarettes have been smoked. This doesn’t necessarily mean that the birds use cigarette butts as an adaptive anti-parasite strategy. Cellulose in the butts is an effective thermal insulator so any anti-parasite effects may be a fortuitous coincidence. The authors suggest that future behavioural choice tests could be used to determine whether birds can distinguish and preferentially include smoked cigarette butts in their constructions.

The paper is an interesting contribution to the growing fields of urban ecological and wildlife research. More than half of the world’s population now lives in urban areas so it is increasingly important to understand the ecological effects of this changing environment. Wildlife and urban areas are not always a happy mix – we have all seen the squished remains of a hedgehog’s attempt to cross a busy road. However, as this paper shows, sometimes urban animals can adopt novel behaviours which appear to have positive consequences.

However, I can’t see the paper being used to counteract anti-cigarette butt litter campaigns any time soon!


Author

Sive Finlay: sfinlay[at]tcd.ie

Photo credit

wikimedia commons
Hippo Critical

800px-Hippopotamus_amphibius_Whipsnade_Zoo

Hippopotami have been the talk of the Trinity College Zoology department’s tea room recently. Mainly because a number of staff are about to embark on a field trip to Kenya with some undergraduate students and hippos have featured highly on the list of possible animals which an encounter with might result in death or injury, I therefore decided to investigate, partly to allay fears but mainly to stir them.

In a recent study by Dunham et al. (2010) they investigated human-wildlife conflicts which have resulted in death or injury. The fact that Hippos are one of the most dangerous animals in Africa is common knowledge (in our tea room anyway), but the good news is that crocodiles are far more dangerous. Oh and lions, lions are really dangerous, but mostly crocodiles. In Mozambique crocodiles have killed more people than all other animals combined. More good news for our would-be travellers, only 55% of hippo attacks resulted in death, whereas the figure is close to 80% for crocodiles and alarmingly even higher for elephants. Though chillingly there have been reports of Hippos abandoning herbivory for a more carnivorous lifestyle.

Overall it is good news, hippos are not in fact that dangerous as long as you can manage to keep away from the water. So our intrepid explorers can relax in their campsite in their tents on the shores of lake Naivasha just remember hippos come onto land at night to feed, so perhaps pitch your tent away from the juicy grass.


Author

Keith McMahon: mcmahok[at]tcd.ie

Photo credit

Wikimedia commons

The undiscovered island

Early ecological research relied on adventurous naturalists striking forth into unknown territory and expanding our knowledge of the natural world. This exploratory work is far from complete and many species new to science are still being identified. However, in order to study and investigate the remaining unexplored frontiers, knowing where they are is a fundamental necessity.

Finding our way around has never been so easy. GPS trackers are readily available; Google maps takes the stress out of navigating unfamiliar cities and Google Earth allows us to look down from above on some of the most remote regions of the world. The works of early cartographers with approximations of coastlines and vague “beyond here there are monsters” warnings can be relegated to historical archives. However, a recent discovery by the research vessel Southern Surveyor during its surveys of the seabed off Australia reminds us not to be so trusting of our highfalutin technology.

Sandy Island featured on weather maps and was depicted on Google Earth as lying halfway between Australia and New Caledonia. However, the 24 by 5 kilometre island was not marked on navigation charts. When the Southern Surveyor diverted its course to investigate the supposed island, they found only empty ocean with a depth of about 1.5km. Records of the phantom island seem to trace back to cartographic errors reported by the whaling ship, Velocity, in 1876. The island has now been removed from Google Maps.

The location of Sandy Island depicted on Google Maps.

From a biodiversity perspective, the non-existent island could have been home to a whole host of unusual and endemic species. The surrounding islands in this region of the South West Pacific are the remaining splinters of Australia’s separation from the ancient super-continent, Gondwana. They have high percentages of endemic species with New Caledonia recognised as one of the 25 global biodiversity hotspots. However, human colonisation of the Pacific islands caused significant biodiversity loss which continues today. If Sandy Island had existed, we can only speculate about the number of weird and wonderful creatures which, in the absence of human threats, could have called the island home.

Inaccurate maps from the 19th Century aren’t that surprising but it is pretty incredible that in our technologically savvy age an island the size of Manhattan just doesn’t exist! One expedition member commented that the mistake “raises all kinds of conspiracy theories” especially when the CIA is one of the contributing sources to the world coastline database.

I guess this is just a reminder that Google is not omnipotent after all!

Author

Sive Finlay: sfinlay[at]tcd.ie

Photo credit

wikimedia commons